Review Article
Rhizosphere Soil Properties and Growth Performance of Fritillaria thunbergii under Continuous Cropping 

 Author Correspondence author
Molecular Soil Biology, 2026, Vol. 17, No. 5
Received: 01 Jan., 1970 Accepted: 01 Jan., 1970 Published: 12 Oct., 2026
Fritillaria thunbergii Miq. is an important medicinal plant with high economic and pharmacological value; however, its production is increasingly constrained by continuous cropping obstacles caused by long-term monoculture practices. Continuous cropping can induce complex changes in rhizosphere soil environments, including nutrient imbalance, soil physicochemical degradation, microbial community dysbiosis, accumulation of autotoxic compounds, and increased pathogen pressure, ultimately leading to reduced plant growth, bulb yield, and medicinal quality. This review systematically summarizes the effects of continuous cropping on rhizosphere soil properties and growth performance of F. thunbergii, with emphasis on soil physicochemical characteristics, microbial ecological changes, plant physiological responses, and soil-plant interaction mechanisms. Continuous cropping alters key soil parameters, including pH, organic matter content, nutrient availability, soil structure, and enzyme activities, which directly affect root development and nutrient acquisition. Meanwhile, prolonged cultivation reshapes rhizosphere microbial communities by reducing beneficial microorganisms and enriching soil-borne pathogens, thereby disrupting microbial-mediated nutrient cycling and disease suppression functions. At the plant level, continuous cropping stress inhibits root growth, reduces photosynthetic capacity, induces oxidative stress, and negatively affects bulb accumulation and medicinal compound biosynthesis. The interaction between soil degradation, microbial imbalance, and plant physiological stress forms a major ecological mechanism underlying continuous cropping obstacles in F. thunbergii. A case study approach is presented to analyze dynamic changes in rhizosphere soil properties and plant growth responses across different continuous cropping years, highlighting key environmental drivers influencing productivity decline. Furthermore, this review discusses sustainable strategies for overcoming continuous cropping limitations, including crop rotation, organic amendments, beneficial microbial inoculation, and precision rhizosphere management. Future research integrating multi-omics technologies, microbiome engineering, and intelligent agricultural approaches will provide new opportunities for improving soil health and achieving sustainable production of Fritillaria thunbergii.
1 Introduction
Fritillaria thunbergii is an economically important medicinal plant whose bulb has been used in China for more than two millennia and remains widely valued for relieving cough and clearing the lungs. Its medicinal importance extends beyond traditional use because modern studies describe broad pharmacological activities, including antitussive, expectorant, anti-inflammatory, antioxidant, anticancer, and other bioactive effects that are attributed largely to its rich alkaloid-centered phytochemistry (Nile et al., 2021). The bulb is the medicinal organ and contains steroidal alkaloids, polysaccharides, flavonoids, and other constituents that determine commercial quality, making cultivation practices central not only to yield but also to therapeutic value (Li et al., 2019). This production challenge has intensified as market demand has risen while wild resources have declined and cultivation systems have become more intensive, increasing pressure to sustain both biomass accumulation and medicinal ingredient content under field conditions (Qu et al., 2022; Liu et al., 2025).
Continuous cropping is a major barrier to sustainable medicinal-plant production because it alters the rhizosphere through interacting physical, chemical, and biological processes rather than through a single cause (Haq et al., 2023). Across medicinal plants, continuous cropping obstacles are associated with nutrient imbalance, soil acidification, shifts in enzyme activity, autotoxic root exudate accumulation, loss of beneficial microorganisms, and enrichment of pathogens, which together reduce plant vigor, yield, and quality (Liao and Xia, 2024). Reviews focused on medicinal-plant rhizospheres further show that secondary metabolites released under repeated monoculture can accumulate to inhibitory concentrations, destabilize microbial community structure, and amplify disease risk through species-specific plant-soil feedbacks (Yuan et al., 2022). Similar patterns have been documented in other continuous-cropping systems, where long-term monoculture changes microbial composition and functional pathways related to nutrient cycling, reinforcing the view that rhizosphere degradation is a core mechanism of cropping obstacle formation (Pang et al., 2021).
For F. thunbergii specifically, available evidence already indicates that continuous cropping reshapes rhizosphere soil properties in ways consistent with these broader medicinal-plant obstacles (Haq et al., 2025). Field work comparing 1-, 2-, and 4-year cultivation showed that longer continuous cropping reduced available N, P, and K, lowered soil pH, decreased bacteria and actinomycetes, increased fungi, reduced urease and catalase activities, and coincided with accelerated membrane lipid peroxidation and clear declines in bulb biomass and root system development (Gong et al., 2024). At the same time, newer studies in F. thunbergii show that rhizosphere conditions are not merely passive indicators of decline but active regulators of plant performance, because management with shading, potassium, biochar, or organic fertilizer can improve soil nutrient status, restructure microbial communities, suppress pathogenic fungi, and increase bulb yield and total alkaloid accumulation (Liu et al., 2026). These findings support the idea that rhizosphere ecological regulation is a plausible pathway for overcoming continuous-cropping injury in this species (Wang et al., 2026).
However, important knowledge gaps remain in understanding how rhizosphere regulation mediates growth performance of F. thunbergii under continuous cropping. Current work on this species has focused largely on cultivation inputs and medicinal alkaloid accumulation, and although transcriptomic, metabolomic, and fertilization studies have begun to identify candidate genes and pathways linked to steroidal alkaloid biosynthesis, the synthesis pathway is still described as not fully clear and the effects of cultivation conditions on yield-quality coordination remain insufficiently resolved (Huang et al., 2024). More broadly, continuous-cropping research across medicinal plants still lacks integrated analyses that simultaneously connect rhizosphere physicochemical traits, microbial community succession, soil metabolites, and host growth responses across cropping years (Li et al., 2024). Because soil pH, carbon, nitrogen availability, and microbial functional shifts repeatedly emerge as key drivers in other continuous-cropping systems, a focused study of rhizosphere soil properties and plant growth in continuously cropped F. thunbergii is needed to clarify the mechanisms of obstacle formation and to provide an evidence base for sustainable soil management and quality-oriented production (Wang et al., 2026).
2 Effects of Continuous Cropping on Rhizosphere Soil Physicochemical Properties
2.1 Changes in soil physical characteristics under continuous cropping
Continuous cropping changes the physical status of rhizosphere soil by disrupting the microenvironment that supports root growth, water retention, aeration, and microbe-soil exchange. Reviews of medicinal-plant systems identify moisture, water-holding capacity, compaction, bulk density, porosity, temperature, and related microclimatic factors as part of the soil physicochemical properties affected under continuous cropping, indicating that physical deterioration is a recurring component of cropping obstacles rather than a secondary consequence alone (Liao and Xia, 2024). Because these physical traits regulate oxygen diffusion, nutrient mobility, and root penetration, their deterioration likely amplifies the effects of nutrient imbalance and microbial dysbiosis in continuously cropped fields (Haq et al., 2023).
Although direct measurements of bulk density and porosity are still limited for F. thunbergii, species-specific evidence shows that prolonged continuous cropping significantly reduced plant biomass, root length, and root surface area, implying a progressively less favorable rhizosphere physical environment for root exploration and uptake (Huang et al., 2025). Comparable medicinal-plant studies further show that continuous cropping degrades the soil environment together with crop performance, supporting the interpretation that physical deterioration in the rhizosphere is functionally tied to reduced growth and weakened belowground development.
2.2 Alterations in soil chemical properties and nutrient availability
Chemical changes in the rhizosphere are among the most consistently reported effects of continuous cropping. In F. thunbergii, increasing years of cultivation significantly decreased available N, P, and K while soil pH showed a declining trend, indicating simultaneous nutrient depletion and acidification in the root zone (Gong et al., 2024). This pattern is widely reported across continuous-cropping systems, where reduced pH impairs nutrient use efficiency and contributes to broader nutrient imbalance even when some individual nutrient pools accumulate rather than decline (Zhao et al., 2021).
The direction of nutrient change is not identical across species, but the underlying outcome is consistent: continuous cropping destabilizes nutrient balance and increasingly couples soil chemistry to microbial shifts. For example, Codonopsis pilosula showed declining pH with rising total phosphorus and available potassium across cropping years, whereas Panax ginseng showed lower pH, TN, HN, and OM but higher TP, TK, AP, and AK under continuous cropping, together illustrating that imbalance can involve either depletion or accumulation depending on crop and management history (Chen et al., 2023). Similar long-term results in Fritillaria cirrhosa and tobacco indicate that pH, alkaline nitrogen, and soil organic carbon are key drivers of rhizosphere microbial composition, underscoring that chemical deterioration is central to the continuous-cropping obstacle rather than merely correlative (Gao et al., 2024).
2.3 Accumulation of soil phenolic compounds and autotoxic substances
Accumulation of phenolic compounds and other autotoxins is a major mechanism by which continuous cropping damages rhizosphere function in medicinal plants. Reviews consistently show that under repeated monoculture, medicinal plants release stress-related secondary metabolites that accumulate in soil, produce concentration-dependent autotoxic effects, and destabilize rhizosphere microbial communities by suppressing beneficial microbes and favoring harmful ones (Yuan et al., 2022). This mechanism is also conceptually important for medicinal plants because the biochemical similarity between pharmaceutical active substances and autotoxic allelochemicals has long been proposed as a basic reason why these species are especially prone to continuous-cropping obstacles (Haq et al., 2023).
Evidence from related medicinal plants shows that the specific compounds involved are often phenolic acids, though other organic compounds can contribute. In Polygonatum odoratum, phenolic acid contents were significantly higher in continuous-cropping soil and coincided with lower available N, P, and K, while in continuously cropped tobacco, phenolic acids increased significantly and were negatively correlated with soil pH, suggesting that acidification and autotoxin accumulation reinforce each other (Ni et al., 2021). Studies of Panax notoginseng, Rehmannia glutinosa, Pinellia ternata, and Fritillaria taipaiensis further identify vanillic acid, p-hydroxybenzoic acid, ferulic acid, benzoic acid, palmitic acid, stearic acid, and related compounds as autotoxic or pathogen-promoting metabolites, and show that their accumulation patterns can vary with cropping duration and fertilizer regime (Bao et al., 2022; Yang et al., 2025).
3 Rhizosphere Microbial Community Responses under Continuous Cropping Conditions
3.1 Changes in rhizosphere microbial diversity and community structure
Continuous cropping consistently reshapes rhizosphere microbial diversity and community structure, although the direction of diversity change varies with host species, cropping duration, and soil context. In Fritillaria taipaiensis, long-term single planting did not significantly change Chao1 or ACE richness indices, but Shannon and Simpson indices declined with cultivation year, while beta diversity first decreased and then increased, indicating progressive loss of community evenness and greater between-sample differentiation over time (Zhou et al., 2022). In Fritillaria unibracteata, metagenomic profiling likewise showed significant compositional divergence among one-, two-, and three-year cultivation groups, with bacterial alpha diversity declining significantly after three years, supporting the view that prolonged continuous cropping drives measurable restructuring of the rhizosphere microbiome (Liu et al., 2023).
Evidence from other Fritillaria species and medicinal plants suggests that this restructuring often extends beyond diversity indices to simplification of ecological interactions. In Fritillaria cirrhosa, continuous cultivation altered both bacterial and fungal communities, and after 10 years the number of links in bacterial and fungal co-occurrence networks was markedly lower than in non-continuous soil, indicating a simpler and less compact microbial community structure (Gao et al., 2024). A similar pattern was reported in long-term continuous tobacco and patchouli systems, where continuous cropping significantly changed rhizosphere microbial composition and reduced community stability, implying that sustained monoculture weakens the resilience of rhizosphere microbial assemblages across medicinal and non-medicinal crops.
3.2 Beneficial microorganisms and pathogenic microbial enrichment
A recurrent feature of continuous cropping is the decline of beneficial microorganisms that support nutrient acquisition and disease suppression, together with the enrichment of potentially harmful taxa. In Fritillaria cirrhosa, successively cropped soils showed significant reductions in beneficial microorganisms such as Sphingomonas, Lysobacter, and Cladosporium, alongside accumulation of harmful microorganisms associated with soil-borne disease, while in Fritillaria taipaiensis dominant genera in first-year soil mainly promoted nutrient status and plant growth but shifted toward pathogen accumulation and soil deterioration with increasing cultivation years (Zhou et al., 2022). Comparable trends appear in Fritillaria unibracteata, where beneficial taxa decreased across cultivation years while harmful microorganisms increased, reinforcing that continuous cropping in Fritillaria tends to replace growth-promoting microbiota with stress- and disease-associated assemblages (Liu et al., 2023).
Pathogen enrichment under continuous cropping is also linked to reduced plant health and greater disease risk. In diseased rhizosphere soil of Fritillaria ussuriensis, microbial diversity was lower than in healthy soil, while Fusarium and Humicola increased significantly and beneficial indicators such as RB41 and Arthrobacter were most abundant in healthy soil, directly linking microbial imbalance to wilt severity (Jiao et al., 2022). More broadly, reviews and cross-system studies conclude that autotoxin accumulation and repeated monoculture increase pathogenic microbes while reducing beneficial populations, and in Fritillaria pallidiflora replant soil, phthalate allelochemicals were strongly correlated with Fusarium abundance, showing how chemical and microbial shifts can reinforce one another during replant disease development (Haq et al., 2025).
3.3 Microbial functional changes and soil ecological processes
Changes in rhizosphere microbial communities under continuous cropping are not only taxonomic but also functional, with important consequences for nutrient cycling and soil ecological processes. In continuous tobacco, microbial and gene-based functional analyses indicated that rhizosphere microbiota may regulate soil nutrients through iron respiration, sulfur respiration, and prokaryotic carbon fixation pathways, while changes in community structure were closely related to soil urease, active organic carbon, and available iron (Yang et al., 2025). In continuous sugarcane, metagenomic analysis further showed significant reduction of bacteria associated with nitrogen and sulfur cycling and decreased abundance of nitrogen translocation and sulfate-reduction genes, linking functional losses directly to lower soil nutrient availability and yield decline (Pang et al., 2021).
Studies in perennial medicinal plants indicate that this functional reshaping contributes to broader ecological degradation of continuously cropped soils. In Rhodiola crenulata, continuous cultivation reduced soil multifunctionality by about 46% from the first to the fourth year, while bacterial carbon and nitrogen cycling functions declined and sulfur cycling and stress-response functions increased, indicating a shift from nutrient-supporting to stress-adapted microbial functioning (Jia et al., 2026). In intensively cultivated Fritillaria pallidiflora, continuous cropping increased bacterial-fungal cross-domain network complexity but strongly reduced soil quality and ecological sustainability, and fungal communities came to dominate resource-acquisition and competitive functions, suggesting that altered microbial interactions themselves become part of the mechanism driving long-term soil degradation (Dong et al., 2025).
4 Growth Performance and Physiological Responses of Fritillaria thunbergii under Continuous Cropping
4.1 Effects on plant growth and biomass accumulation
Continuous cropping clearly suppresses the vegetative growth of F. thunbergii. A field study comparing 1-, 2-, and 4-year cropping showed that plant biomass, root length, and root surface area all declined significantly as continuous-cropping duration increased, indicating progressive inhibition of belowground development and whole-plant growth (Yin et al., 2023). This pattern is consistent with broader observations in Fritillaria cultivation that repeated planting in the same field leads to short plants, small bulbs, and poor performance, linking rhizosphere deterioration directly to biomass loss (Zhou et al., 2022).
Evidence from cultivation-year studies shows that growth reduction under continuous cropping does not simply reflect normal developmental variation. In F. thunbergii, rapid bulb filling begins about 32 days after sprouting and bulb growth is completed in about 72 days, but the proportion of bulbs exceeding 5 g declines from 89% at one year to 77% at three years, suggesting that repeated cultivation increasingly limits bulb expansion even when plants complete their developmental program. Related work in other medicinal crops under continuous cropping likewise reports inhibited growth, including higher dead-seedling rates and structural damage in roots, supporting the view that biomass decline in F. thunbergii is part of a broader syndrome of monoculture stress in medicinal plants (Xu et al., 2025).
4.2 Physiological responses to continuous cropping stress
The physiological response of F. thunbergii to continuous cropping is dominated by oxidative stress. Under increasing continuous-cropping duration, membrane lipid peroxidation accelerated, while superoxide dismutase and peroxidase activities declined, showing that the antioxidant defense system weakened as rhizosphere stress intensified (Hang et al., 2023). Similar responses in other continuously cropped medicinal plants include increased reactive oxygen species, elevated malondialdehyde, and altered osmotic-regulation metabolites, which together indicate that redox imbalance is a common physiological consequence of successive planting (Gao et al., 2024).
This stress response likely integrates nutrient limitation, pathogen pressure, and disrupted redox regulation rather than operating through a single pathway. In Pinellia ternata, continuous cropping altered expression of genes involved in photosynthesis, chlorophyll biosynthesis, defense response, plant-pathogen interaction, and phytohormone signaling, while phosphorus depletion and pathogen damage were inferred to be key causes of the cropping obstacle (Hang et al., 2023). A broader physiological analysis in Qingke similarly showed that continuous cropping elevated reactive oxygen species across development and reduced total antioxidant capacity, reinforcing that persistent oxidative burden can translate into growth suppression and lower productivity when antioxidant systems fail to compensate (Figure 1) (Gao et al., 2024).
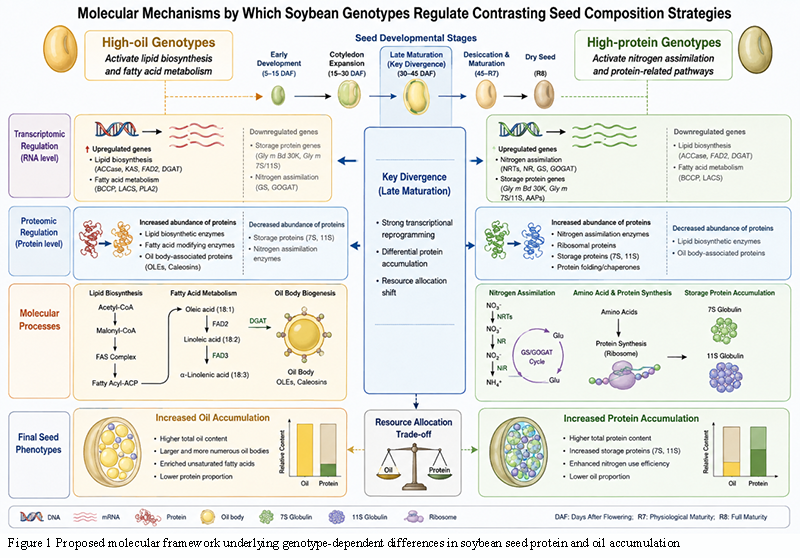 Figure 1 Proposed molecular framework underlying genotype-dependent differences in soybean seed protein and oil accumulation |
4.3 Effects on bulb yield and medicinal quality formation
Continuous cropping affects not only bulb yield but also the formation of medicinal quality, creating a central production trade-off for F. thunbergii. In continuously planted Fritillaria fields, yield and quality decline together, and in F. cirrhosa the reduction becomes especially severe after more than 5 years of continuous cultivation, when yield falls by more than 80% (Yin et al., 2023). Because the medicinal value of F. thunbergii bulbs depends mainly on steroidal alkaloids such as peimine and peiminine, any cultivation practice that depresses bulb development or destabilizes metabolism can directly reduce commercial and pharmacological quality (Yin et al., 2023).
At the same time, recent intervention studies show that yield and medicinal quality can be at least partly recovered when rhizosphere conditions are improved. Reductive soil disinfestation combined with iron amendment increased F. thunbergii yield by 24.2% and peimisine content by 49.3%, indicating that soil remediation can simultaneously improve productivity and active-ingredient accumulation. Likewise, optimized cultivation management altered quality formation: organic fertilizer produced a yield of 2.70 kg/m2 together with higher peimine and peiminine contents, while shading plus potassium increased active ingredients by about 20.71% and partially alleviated biomass reduction, showing that medicinal quality formation is highly responsive to rhizosphere and environmental regulation (Huang et al., 2024; Liu et al., 2025).
5 Interactions between Rhizosphere Soil Properties and Plant Growth Performance
5.1 Soil-root interaction mechanisms under continuous cropping
Under continuous cropping, soil-root interactions in medicinal plants shift from a mutually supportive system toward a stress-amplifying rhizosphere feedback loop. The rhizosphere functions as the main hub for material exchange and signaling among roots, soil, and microorganisms, but repeated planting causes root exudates to release autotoxins that alter soil physicochemical properties and restructure microbial communities, thereby weakening plant vigor (Haq et al., 2025). This mechanism is directly relevant to F. thunbergii, because continuous cropping progressively reduced root length and root surface area while simultaneously inducing nutrient deficiency, acidification, microbial imbalance, and oxidative stress in the rhizosphere, indicating that root performance declines as the soil environment becomes less favorable for absorption and defense (Liao and Xia, 2024).
Root-mediated feedback under continuous cropping is not driven by exudation alone, but by the coupled response of roots and microbes to repeated stress exposure. Studies in Panax notoginseng show that plants primarily communicate with soil through root exudates, which directly or indirectly reshape microbial community structure, while studies in green pepper further show that continuous-cropping duration alters exudate composition and that accumulated compounds can inhibit root development and vitality through rhizosphere feedback inhibition (Bao et al., 2022). A similar process likely operates in Fritillaria systems, where increasing planting years have been associated with a shift from high-fertility bacterial-type soil toward low-fertility fungal-type soil, a transition that increases pathogen risk and intensifies root-zone stress (Li et al., 2025).
5.2 Relationships between soil nutrients, microbial communities, and plant growth
The relationship between soil nutrients, microbial communities, and plant growth under continuous cropping is strongly interactive rather than sequential. Continuous cropping changes pH, carbon, nitrogen, and available nutrient pools, and these variables in turn drive microbial community assembly, with pH, alkaline nitrogen, and soil organic carbon repeatedly identified as major determinants of rhizosphere microbial composition (Ding et al., 2024; Liu et al., 2025). In F. thunbergii, declining available N, P, and K and lower pH coincide with reduced biomass and root growth, supporting the interpretation that nutrient imbalance and microbial dysbiosis jointly limit plant performance rather than acting as isolated constraints (Xia et al., 2025).
Microbial communities also feed back on plant growth by regulating nutrient transformation, nutrient accessibility, and stress resistance. Soil microorganisms can decompose toxic compounds but can also generate additional phytotoxic products during allelopathic residue breakdown, and rhizosphere microbes influence nutrient contents through functions such as iron respiration, sulfur respiration, and prokaryotic carbon fixation (Yang et al., 2025). The growth consequence of these linkages is evident across systems: enzyme activity, microbial diversity, and nitrogen- and phosphorus-related availability show positive feedbacks with crop performance in Curcuma kwangsiensis, while beneficial nutrient-mobilizing and nitrogen-fixing bacteria promote root-zone extension and nutrient absorption efficiency in cowpea (Huang et al., 2025; Zhu et al., 2025).
5.3 Integrated mechanisms of continuous cropping obstacles formation
Current evidence supports an integrated mechanism in which continuous-cropping obstacles arise from the convergence of autotoxic accumulation, soil degradation, and microbial dysbiosis. Reviews of medicinal plants identify three recurring core drivers-autotoxicity, soil nutrient imbalance, and disrupted microbial communities—and emphasize that these drivers act through an interconnected plant-soil-microbe interaction system rather than through a single causal pathway (Xu et al., 2025). This integrated view is reinforced by system-level studies showing that the core mechanism is a chain reaction in which soil nutrient pool imbalance induces functional shifts in microbial communities, leading to synchronized declines in plant growth and defense (Li et al., 2025).
A plausible mechanistic model for F. thunbergii is therefore that repeated planting alters root exudation, promotes the buildup of phenolic or other autotoxic metabolites, acidifies and imbalances the rhizosphere, reduces beneficial microbial functions, and enriches pathogens, together suppressing root activity, nutrient uptake, and biomass accumulation. Evidence from Eleutherococcus senticosus supports a “pathogen invasion-metabolite accumulation-coexistence of resistance and autotoxicity” framework, while work in Codonopsis pilosula shows that continuous-cropping obstacles can be traced to the combined effects of nutrient imbalance and autotoxic substance accumulation (Li et al., 2024; Jia et al., 2026). Overall, continuous-cropping obstacles in F. thunbergii are best understood as an emergent rhizosphere syndrome produced by tightly coupled changes in soil chemistry, microbial ecology, and root physiological function.
6 Case Study: Comprehensive Analysis of Rhizosphere Soil Changes and Growth Responses of Fritillaria thunbergii under Different Continuous Cropping Years
6.1 Experimental design and evaluation indicators
A practical case-study framework for F. thunbergii continuous-cropping research combines multi-year field comparison with synchronized rhizosphere and plant measurements. In the species-specific field study, rhizosphere soil properties, microbial flora, enzyme activities, and plant growth were compared across 1-, 2-, and 4-year continuous-cropping treatments, directly linking cropping duration to both soil and plant responses (Yin et al., 2023). This design is strengthened by evidence from related Fritillaria systems showing that year-gradient sampling is suitable for tracking rhizosphere succession, as one- to five-year rhizosphere soils in F. taipaiensis were compared using replicated field plots and integrated soil-microbial analyses (Zhou et al., 2022).
Sampling protocols used in F. thunbergii and related medicinal-plant studies indicate that representative rhizosphere assessment requires plot-level replication, standardized root-zone collection, and parallel processing for physicochemical, enzymatic, and microbial analyses. For F. thunbergii, regional rhizosphere studies sampled multiple plants per site and separated tightly adhering soil from bulk soil to characterize pH, organic matter, enzyme activity, and bacterial community structure, while continuous-cropping remediation trials stored split samples for soil properties, microbial activity, and DNA-based community analysis (Figure 2) (Yin et al., 2023). Accordingly, key evaluation indicators in a comprehensive case study should include soil pH, available N, P, and K, organic matter, urease and catalase activities, bacterial and fungal community composition, root length, root surface area, biomass, bulb yield, and alkaloid-related quality traits.
 Figure 2 Experimental framework for evaluating continuous cropping effects in Fritillaria thunbergii using multi-year field comparisons |
6.2 Dynamic changes in soil properties and plant growth during continuous cropping
Across continuous-cropping years, the clearest dynamic in F. thunbergii is progressive rhizosphere deterioration accompanied by growth suppression. As planting duration increased from 1 to 4 years, available N, P, and K decreased significantly, soil pH declined, bacteria and actinomycetes decreased, fungi increased, and urease and catalase activities fell, while plant biomass, root length, and root surface area also declined significantly (Zhou et al., 2022). This trajectory agrees with broader Fritillaria evidence that long-term planting shifts the rhizosphere from a high-fertility bacterial type toward a low-fertility fungal type, which is typically associated with weaker plant performance and greater continuous-cropping pressure (Liao and Xia, 2024).
Year-dependent shifts also appear to follow a cumulative ecological pattern rather than a simple linear loss of fertility. In F. unibracteata, rhizosphere microbiome composition differed significantly among one-, two-, and three-year cultivation groups, with dominant genera shifting from Pseudomonas and Botrytis in the first year to Mycolicibacterium and Pseudogymnoascus by the third year, while beneficial microorganisms decreased and harmful microorganisms increased (Liu et al., 2023). A similar year-gradient pattern in F. taipaiensis showed that Shannon and Simpson diversity declined with cultivation year and that the dominant genera progressively shifted from taxa associated with nutrient improvement and plant growth to taxa reflecting pathogen accumulation and soil nutritional deterioration, with soil pH emerging as the strongest correlate of bacterial community composition (Zhou et al., 2022).
6.3 Identification of key drivers and potential improvement strategies
The combined evidence identifies soil acidification, nutrient imbalance, microbial dysbiosis, and autotoxic metabolite accumulation as the main drivers of continuous-cropping obstacles. Reviews of medicinal plants describe continuous-cropping failure as a rhizosphere process in which root-exuded autotoxins alter soil properties, reduce beneficial microorganisms, and enrich pathogenic populations, while Fritillaria studies further show that alkaline hydrolytic nitrogen and available phosphorus can alter soil pH and thereby drive microbial-community change and soil-health decline (Liao and Xia, 2024). Related Fritillaria evidence also suggests that changes in volatile compounds and other metabolites participate in microbiome restructuring, because continuous monoculture reduced rhizosphere VOC diversity and phthalates were strongly associated with Fusarium abundance and disease-promoting community shifts (Cao et al., 2025).
Potential improvement strategies should therefore target soil chemistry, microbial structure, and pathogen pressure together rather than separately. In F. thunbergii, reductive soil disinfestation with potato peel increased soil pH, organic matter, microbial activity, K, and Ca, enriched beneficial microbes, reduced potential pathogens, and when combined with iron amendment increased yield by 24.2% and peimisine content by 49.3% (Yin et al., 2023). More recent evidence further shows that biochar plus organic fertilizer increased available nutrients and soil organic matter, enhanced microbial diversity and nutrient-cycling genes, reduced pathogenic fungi, and improved both yield and total alkaloid content, supporting integrated rhizosphere regulation as a credible strategy for alleviating continuous-cropping obstacles in F. thunbergii (Liu et al., 2026).
7 Sustainable Management Strategies for Alleviating Continuous Cropping Obstacles
7.1 Crop rotation and diversified cropping systems
Crop rotation and diversified cropping systems are among the most practical strategies for alleviating continuous-cropping obstacles because they interrupt host-specific pathogen buildup and reassemble a more balanced rhizosphere microbiome. In medicinal plant systems, rotation significantly improved agronomic traits, yield, and quality, while suppressing Fusarium and modulating soil nutrients, enzyme activities, microbial communities, and rhizosphere metabolites; more broadly, rotation and related ecological practices are recommended to address soil health decline caused by continuous cultivation (Gao et al., 2024; Chen et al., 2025).
The likely value of this approach for Fritillaria thunbergii is strengthened by mechanistic work showing that, compared with rotation, intensive monocropping weakens the rhizosphere’s capacity to prevent pathogen invasion and promotes soil-borne disease development. More generally, native microbiome steering through crop rotation, host selection, or soil amendments is increasingly viewed as a feasible way to improve persistence and ecological compatibility, especially where stable establishment of introduced strains is uncertain (Zhou et al., 2023; Fouad et al., 2026).
7.2 Organic amendments and rhizosphere environment improvement
Organic amendments improve rhizosphere conditions by restoring soil fertility, buffering adverse physicochemical changes, and promoting beneficial microbial functions. In F. thunbergii, reductive soil disinfestation with potato peel significantly reduced salinity and increased soil pH, microbial activity, organic matter, and K and Ca contents, while also enriching beneficial microbes and reducing potential pathogens; these changes were accompanied by improved yield and quality (Yin et al., 2023).
Recent field evidence further shows that combining biochar with organic fertilizer provides a broader microecological benefit than fertilization alone. In understory F. thunbergii, this combined treatment significantly increased yield and total alkaloid content, improved available nutrients and soil organic matter, increased beneficial bacteria, reduced pathogenic fungi, and enhanced genes involved in C, N, P, and S cycling, indicating that amendment-driven rhizosphere repair can support both productivity and medicinal quality formation (Liu et al., 2026).
7.3 Biological regulation and precision Rhizosphere management
Biological regulation offers a targeted complement to rotation and organic amendment by directly rebuilding disease-suppressive and growth-promoting functions in the rhizosphere. In F. thunbergii, wild-enriched Penicillium strains isolated from the rhizosphere showed dual effects on disease suppression and plant growth promotion through phosphate solubilization, siderophore production, pathogen antagonism, and induction of defense-related genes; in parallel, Fritillaria reviews have emphasized the need to develop safe, efficient, pollution-free microbial agents to improve soil environment, yield, and quality (Zhou et al., 2022; Cai et al., 2026).
Precision rhizosphere management is increasingly framed as matching the intervention to the crop-soil context rather than relying on one universal product. Reviews of microbial biocontrol and microbiome engineering indicate that synthetic consortia can integrate complementary functions such as nitrogen fixation, phosphate solubilization, siderophore production, and stress buffering, but they require careful formulation, persistence assessment, and multi-site validation; correspondingly, microbial inoculants in other medicinal and continuous-cropping systems have already increased biomass and quality by reshaping microbial communities and reducing pathogen-associated functions (Iqbal, 2026; Wang et al., 2026).
8 Conclusions and Future Perspectives
Under continuous cropping, the rhizosphere of F. thunbergii shows a consistent pattern of physicochemical and biological deterioration. Direct evidence from F. thunbergii indicates that increasing cropping years reduce available N, P, and K, lower soil pH, decrease bacteria and actinomycetes, increase fungi, and weaken urease and catalase activities, while broader Fritillaria syntheses describe this process as a shift from a high-fertility bacterial type to a low-fertility fungal type rhizosphere. This pattern is consistent with rhizosphere-scale observations that F. thunbergii roots modify local soil conditions, with lower pH, organic carbon, phosphatase, and urease in rhizosphere soil than in bulk soil, indicating active root-soil feedbacks that likely intensify under repeated planting. Evidence from other Fritillaria species and continuous-cropping systems suggests that these rhizosphere changes are cumulative and mechanistically linked to microbial restructuring and metabolite disturbance. In F. taipaiensis, bacterial diversity declined with cultivation year and pH was the strongest factor associated with community composition, while in F. unibracteata beneficial microorganisms decreased and harmful microorganisms increased over successive years. Lower-ranked but relevant studies further show that continuous cropping can enrich Fusarium in F. thunbergii fields and that declining rhizosphere VOC diversity, together with phthalate accumulation, can restructure microbiomes and increase disease pressure in replanted Fritillaria systems.
The practical implication is that improving F. thunbergii growth and medicinal quality requires restoring soil chemistry and microbial ecology together rather than treating nutrient supply alone. In F. thunbergii, reductive soil disinfestation with potato peel increased pH, microbial activity, organic matter, K, and Ca, enriched beneficial microbes, reduced pathogens, and improved yield and quality, while biochar plus organic fertilizer increased available nutrients, soil organic matter, beneficial bacteria, and total alkaloid content. These outcomes fit the broader conclusion that soil quality and microbial community improvement are core drivers of higher yield and medicinal value in F. thunbergii cultivation. Management should also account for the trade-off between biomass production and medicinal compound accumulation. Fertilization studies show that organic fertilizer can increase peimine, peiminine, and yield in F. thunbergii, and transcriptomic evidence links this response to ABA signaling and candidate genes for steroidal alkaloid accumulation. Likewise, shading combined with potassium application can mitigate biomass loss while enhancing active ingredient accumulation through rhizosphere microecological regulation, suggesting that precision adjustment of the root-zone environment can improve both bulb productivity and medicinal quality.
Future research should move from descriptive surveys toward causal, integrated, and predictive studies of the F. thunbergii rhizosphere. Current evidence shows that continuous-cropping obstacles emerge from interacting changes in soil pH, nutrients, metabolites, and microbial communities, yet several studies explicitly note that the interaction between soil physicochemical factors and microbial dynamics remains insufficiently resolved and that root exudate-soil-microbe mechanisms require deeper study. A priority is therefore to combine long-term field trials with metagenomics, metabolomics, transcriptomics, and ecological network analysis to identify the key drivers that convert a healthy rhizosphere into a disease-prone one. A second priority is to develop stable biological regulation strategies tailored to F. thunbergii production systems and regional microbiomes. Wild-rhizosphere mining has already identified Penicillium strains with phosphate solubilization, siderophore production, pathogen antagonism, and defense induction, validating plant microbiome rewilding as a promising control strategy. At the same time, population-scale microbiome work shows strong geographic structuring and environmental selection in F. thunbergii rhizosphere communities, implying that future inoculants and management programs should be site-adapted rather than universal.
Acknowledgments
I extend my sincere gratitude to the anonymous reviewers for their valuable and insightful comments, which have greatly strengthened this paper.
Conflict of Interest Disclosure
The author affirms that this research was conducted without any commercial or financial relationships that could be construed as a potential conflict of interest.
Bao L., Liu Y., Ding Y., Shang J., Wei Y., Tan Y., and Zi F., 2022, Interactions between phenolic acids and microorganisms in rhizospheric soil from continuous cropping of Panax notoginseng, Frontiers in Microbiology, 13: 791603.
https://doi.org/10.3389/fmicb.2022.791603
Cai L., Sun J., Li H., Wang C., Zhang M., Shao Q., and Wang Z., 2026, A novel internal reference microorganism-based method reveals wild-enriched Penicillium for enhancing growth and disease resistance in Fritillaria thunbergii, Frontiers in Microbiology, 17: 1746815.
https://doi.org/10.3389/fmicb.2026.1746815
Cao S., Li Y., Dong J., Qin B., Yang G., Yin Y., and Zhao W., 2025, Decline in rhizosphere VOC diversity drives microbiome restructuring inducing Fritillaria pallidiflora replant disease, Industrial Crops and Products, 234: 121622.
https://doi.org/10.1016/j.indcrop.2025.121622
Chen F., Xie Y., Jia Q., Li S., Li S., Shen N., Jiang M., and Wang Y., 2023, Effects of the continuous cropping and soilborne diseases of Panax ginseng C.A. Meyer on rhizosphere soil physicochemical properties, enzyme activities, and microbial communities, Agronomy, 13(1): 210.
https://doi.org/10.3390/agronomy13010210
Chen Q.H., Mushtaq W., Wang X., Liao Z., Li J., Xiao S., Miao Y., and Liu D., 2025, Crop rotation alleviates continuous cropping obstacles in Chrysanthemum morifolium production by regulating rhizosphere soil microbial communities and metabolites, Environmental Microbiome, 20(1): 90.
https://doi.org/10.1186/s40793-025-00754-x
Ding M., Dai H., He Y., Liang T., Zhai Z., Zhang S., Hu B., Cai H., Dai B., Xu Y., and Zhang Y., 2024, Continuous cropping system altered soil microbial communities and nutrient cycles, Frontiers in Microbiology, 15: 1374550.
https://doi.org/10.3389/fmicb.2024.137455
Dong J., Li Y., Zhao W., Dong H., Sai C., Yang G., Yin Y., Qin B., Li Y., Li G., and Zhao W., 2025, The intensive cultivation of perennially grown Fritillaria pallidiflora Schrenk increases the complexity of bacterial-fungal cross-domain networks but reduces the evaluation of soil quality and ecological sustainability, Industrial Crops and Products, 236: 122088.
https://doi.org/10.1016/j.indcrop.2025.122088
Fouad N.Y., Elzayat E.M., Amr D., El-Khishin D., Radwan K.H., Youssef A., Khalaf A., Ahmed H.A., Radwan E.H., Tawkaz S., and Baum M., 2026, Rhizosphere microbiome engineering for climate-smart agriculture: From synthetic consortia to precision decision support, Microorganisms, 14(5): 1138.
https://doi.org/10.3390/microorganisms14051138
Gao D., Gao X., Wang Y., Huo H., Wu Y., Yang Z., Zhang H., Yang X., Li F., and Li X., 2024, Effects of long-term continuous cultivation on the structure and function of soil bacterial and fungal communities of Fritillaria cirrhosa on the Qinghai-Tibetan Plateau, Scientific Reports, 14(1): 21291.
https://doi.org/10.1038/s41598-024-70625-x
Gao X., Tan J., Yi K., Lin B., Hao P., Jin T., and Hua S., 2024, Elevated ROS levels caused by reductions in GSH and AsA contents lead to grain yield reduction in Qingke under continuous cropping, Plants, 13(7): 1003.
https://doi.org/10.3390/plants13071003
Gao Y., Zhang J., Sun L., Wang K., and Tang X., 2026, Diversity and distribution of the microbiome in the bulbs and rhizosphere soil of Fritillaria thunbergii, Frontiers in Microbiology, 17: 1752283.
https://doi.org/10.3389/fmicb.2026.1752283
Gong B., He Y., Luo Z.-B., Peng H., Cai H., Zhu Y., Bin J., and Ding M., 2024, Response of rhizosphere soil physicochemical properties and microbial community structure to continuous cultivation of tobacco, Annals of Microbiology, 74(1): 4.
https://doi.org/10.1186/s13213-023-01748-1
Hang Y., Hu T., Tian Y.H., Zhang Y., Shangguan L., Liu M., and Zhang M.S., 2023, Physiological and transcriptomic responses of Pinellia ternata to continuous cropping, Industrial Crops and Products, 205: 117511.
https://doi.org/10.1016/j.indcrop.2023.117511
Haq M.Z.U., Bai Z., Gu G., Liu Y., Yang D., Yang H., Yu J., and Wu Y.G., 2025, Continuous cropping obstacles in medicinal plants: Driven by soil microbial communities and root exudates, Plant Science, 259: 112686.
https://doi.org/10.1016/j.plantsci.2025.112686
Haq M.Z.U., Yu J., Yao G., Yang H., Iqbal H.A., Tahir H., Cui H., Liu Y., and Wu Y.-G., 2023, A systematic review on the continuous cropping obstacles and control strategies in medicinal plants, International Journal of Molecular Sciences, 24(15): 12470.
https://doi.org/10.3390/ijms241512470
Huang L., Liang S., Luo L., Wu M., Fu H.L., and Zhong Z., 2024, Transcriptomic analysis reveals effects of fertilization towards growth and quality of Fritillaria thunbergii bulbus, PLOS One, 19(9): e0309978.
https://doi.org/10.1371/journal.pone.0309978
Huang Z., Wang X., Fan L., Jin X., Zhang X., and Wang H., 2025, Continuous cropping of Tussilago farfara L. has a significant impact on the yield and quality of its flower buds, and physicochemical properties and the microbial communities of rhizosphere soil, Life, 15(3): 404.
https://doi.org/10.3390/life15030404
Iqbal M., 2026, Microbial biocontrol agents and the rhizosphere microbiome: Integrating ecological function and climate resilience in sustainable agriculture, Frontiers in Microbiology, 17: 1771649.
https://doi.org/10.3389/fmicb.2026.1771649
Jia H., Wu X., Deng H., Chen G., Ding R., and Gu R., 2026, Functional reshaping of rhizosphere microorganisms drives the degradation of soil multifunctionality in continuously cultivated Rhodiola crenulata, Industrial Crops and Products, 241: 122837.
https://doi.org/10.1016/j.indcrop.2026.122837
Jiao N., Song X., Song R., Yin D., and Deng X., 2022, Diversity and structure of the microbial community in rhizosphere soil of Fritillaria ussuriensis at different health levels, PeerJ, 10: e12778.
https://doi.org/10.7717/peerj.12778
Li H., Yang Y., Lei J., Gou W., Crabbe M.C., and Qi P., 2024, Effects of continuous cropping of Codonopsis pilosula on rhizosphere soil microbial community structure and metabolomics, Agronomy, 14(9): 2014.
https://doi.org/10.3390/agronomy14092014
Li L., Yang H., Peng D., and Liu R., 2025, Soil acidification and nutrient imbalance mediate fungal community degradation, a key driver of continuous cropping obstacles in Platycodon grandiflorus, Frontiers in Microbiology, 16: 1716243.
https://doi.org/10.3389/fmicb.2025.1716243
Liao J., and Xia P., 2024, Continuous cropping obstacles of medicinal plants: Focus on the plant-soil-microbe interaction system in the rhizosphere, Scientia Horticulturae, 328: 112927.
https://doi.org/10.1016/j.scienta.2024.112927
Liu C., Yu J., Ying J., Hu Z., Liu Z., and Chen S., 2023, Integrated metagenomics and metabolomics analysis reveals changes in the microbiome and metabolites in the rhizosphere soil of Fritillaria unibracteata, Frontiers in Plant Science, 14: 1223720.
https://doi.org/10.3389/fpls.2023.1223720
Liu J., Sheng X., Zhu Z., Zhang K., Yuan Q., Wang H., and Sui N., 2026, Co-application of biochar and organic fertiliser enhances the yield and quality of understory Fritillaria thunbergii Miq. by optimising soil and rhizosphere microecological structure, Industrial Crops and Products, 246: 123387.
https://doi.org/10.1016/j.indcrop.2026.123387
Liu J., Zhu Z., Wang L., Yuan Q., Zhu H., Sheng X., Zhang K., Liang B., Jin H., Wang S., Weng W., Wang H., and Sui N., 2025, Regulation of steroidal alkaloid biosynthesis in bulbs of Fritillaria thunbergii Miq. by shading and potassium application: Integrating transcriptomics and metabolomics analyses, Biology, 14(6): 633.
https://doi.org/10.3390/biology14060633
Liu Z., Ying J., and Liu C., 2024, Changes in rhizosphere soil microorganisms and metabolites during the cultivation of Fritillaria cirrhosa, Biology, 13(5): 334.
https://doi.org/10.3390/biology13050334
Ni X., Jin C., Liu A., Chen Y., and Hu Y., 2021, Physiological and transcriptomic analyses to reveal underlying phenolic acid action in consecutive monoculture problem of Polygonatum odoratum, BMC Plant Biology, 21(1): 362.
https://doi.org/10.1186/s12870-021-03135-x
Nile S.H., Su J., Wu D., Wang L., Hu J., Sieniawska E., and Kai G., 2021, Fritillaria thunbergii Miq. (Zhe Beimu): A review on its traditional uses, phytochemical profile and pharmacological properties, Food and Chemical Toxicology, 153: 112289.
https://doi.org/10.1016/j.fct.2021.112289
Pang Q., Alami M., Yu W., Zhen O., Shu S., Tu D., Alami M.J., and Wang X., 2023, A meta-analysis in nine different continuous cropping fields to find the relationship between plant species and rhizosphere fungal community, Agronomy, 13(7): 1827.
https://doi.org/10.3390/agronomy13071827
Pang Z., Dong F., Liu Q., Lin W., Hu C., and Yuan Z., 2021, Soil metagenomics reveals effects of continuous sugarcane cropping on the structure and functional pathway of rhizospheric microbial community, Frontiers in Microbiology, 12: 627569.
https://doi.org/10.3389/fmicb.2021.627569
Qu A., Wu Q., Su J., Li C., Yang L., Wang Z., Wang Z., Li Z., Ruan X., Zhao Y., and Wang Q., 2022, A review on the composition and biosynthesis of alkaloids and on the taxonomy, domestication, and cultivation of medicinal Fritillaria species, Agronomy, 12(8): 1844.
https://doi.org/10.3390/agronomy12081844
Wang E., Chen C., and Li Q., 2025, Current obstacles for continuous cropping of Panax species and mitigation strategies, Journal of Ginseng Research, 50(1): 1-12.
https://doi.org/10.1016/j.jgr.2025.11.013
Wang Y., Song T., Liang R., Zhang Y., Wang W., Cao L., Li L., and Lin Y., 2026, Microbial inoculants alleviate continuous cropping obstacles in Gynostemma pentaphyllum (Thunb.) Makino by reshaping rhizosphere microbial communities, Industrial Crops and Products, 244: 123231.
https://doi.org/10.1016/j.indcrop.2026.123231
Xia H., Jiang C.-Q., Riaz M., Yu F., Dong Q., Yan Y., Zu C., Zhou C., Wang J., and Shen J., 2025, Impacts of continuous cropping on soil fertility, microbial communities, and crop growth under different tobacco varieties in a field study, Environmental Sciences Europe, 37(1): 5.
https://doi.org/10.1186/s12302-024-01037-x
Xu D., Peng C., Si G., Xu X., Zhao S., You C., and Zhou W., 2025, Soil microbiome dysbiosis and rhizosphere metabolic dysfunction drive continuous cropping obstacles of Codonopsis tangshen, Frontiers in Microbiology, 16: 1628234.
https://doi.org/10.3389/fmicb.2025.1628234
Yang W., Li J., Zhou Y., Wang Y., Wenting W., Zhou N., and Wu Q.-S., 2025, Phenolic acid reduction in Fritillaria taipaiensis rhizosphere via organic fertilization, Plant Signaling and Behavior, 20(1): 2554917.
https://doi.org/10.1080/15592324.2025.2554917
Yin Y., Zhao J., Wang P., You S., Zhou Y., Wong J.W.C., Deng H., Duan G., and Zhu Y., 2023, Reductive soil disinfestation and Fe amendment improve soil microbial composition and Fritillaria production, Applied Microbiology and Biotechnology, 107(21): 6703-6716.
https://doi.org/10.1007/s00253-023-12766-z
Yuan Y., Zuo J., Zhang H., Zu M., and Liu S., 2022, The Chinese medicinal plants rhizosphere: Metabolites, microorganisms, and interaction, Rhizosphere, 22: 100540.
https://doi.org/10.1016/j.rhisph.2022.100540
Zhao Y., Qin X., Tian X., Yang T., Deng R., and Huang J., 2021, Effects of continuous cropping of Pinellia ternata (Thunb.) Breit. on soil physicochemical properties, enzyme activities, microbial communities and functional genes, Chemical and Biological Technologies in Agriculture, 8(1): 43.
https://doi.org/10.1186/s40538-021-00243-6
Zhou N., Mei C.M., Zhu X.Y., Zhao J.J., Ma M.G., and Li W.D., 2022, Research progress of rhizosphere microorganisms in Fritillaria L. medicinal plants, Frontiers in Bioengineering and Biotechnology, 10: 1054757.
https://doi.org/10.3389/fbioe.2022.1054757
Zhou Y., Yang Z., Liu J., Li X., Wang X., Dai C., Zhang T., Carrión V.J., Wei Z., Cao F., Delgado-Baquerizo M., and Li X., 2023, Crop rotation and native microbiome inoculation restore soil capacity to suppress a root disease, Nature Communications, 14(1): 8126.
https://doi.org/10.1038/s41467-023-43926-4
Zhu J., Chen J., Zhang J., Hou Q., Luo K., Li Y., and Feng P., 2025, Response of continuous cropping cowpea and root-zone soil to composite microbial agents: Plant growth promotion and nitrogen-fixing bacterial community regulation, BMC Plant Biology, 25(1): 1537.
https://doi.org/10.1186/s12870-025-07583-7
. HTML
Associated material
. Readers' comments
Other articles by authors
. BioSciAdmin BioSci

Related articles
. Fritillaria thunbergii
. Continuous cropping obstacle
. Rhizosphere soil properties
. Soil microbial community
. Plant-soil interaction
Tools
. Post a comment